Yunwoo Choi and James Vacca, Western Reserve Academy, Hudson, Ohio, United States
Reviewed on 9 May 2026; Accepted on 22 June 2026; Published on 26 October 2026
With help from the 2026 BioTreks Production Team.
Annual U.S. vehicle crashes on snowy and icy roads result in more than 1,300 deaths and 116,800 injuries. However, using chemical road salt to prevent accidents has negative consequences, including corrosion and nearby water contamination. Antifreeze proteins (AFPs) offer a biodegradable, non-corrosive mechanism for inhibiting ice formation without the ecological cost of road salts. Our more eco-friendly design utilizes naturally occurring AFPs to prevent ice formation on road surfaces. This project aimed to create two plasmids for expressing AFPs in E. coli. One plasmid used the pBAD18-Kan vector to express an AFP from L. perenne (perennial ryegrass), while the other used the pUS212 vector to express an AFP from T. molitor (mealworm). Inducible promoters in the two plasmids control both respective genes. Transformed E. coli are lysed and centrifuged to release inclusion bodies. The bodies are then solubilized to recover the expressed AFPs. Extracted AFPs are purified for downstream functionality testing, including ice inhibition under freeze-thaw conditions. In preliminary transformations, robust colony growth was observed for the T. molitor AFP construct, whereas no colonies formed for the L. perenne construct. Consistent with prior results, transformation of the L. perenne AFP construct continued to yield no viable colonies despite optimization of antibiotic selection conditions.
Keywords: Antifreeze proteins, sustainability, Escherichia coli, Tenebrio molitor, Lolium perenne
Authors are listed in alphabetical order. Becky Meyer mentored the group. Please direct all correspondence to mailto:marmersteinv@wra.net.
Background
Winter roads create serious hazards for drivers around the world. In the U.S. alone, icy and snowy conditions contribute to over 1,300 deaths and more than 116,800 injuries from vehicle crashes each year (American Highway Users Alliance, 2018). To make roads safer during the colder months, the U.S. spreads between 15 and 32 million tons of road salt annually (Cary Institute of Ecosystem Studies, n.d.). This salt, mainly sodium chloride, works by lowering water’s freezing point, helping ice melt even when it’s below freezing. Despite its effectiveness, road salt comes with major downsides. It can contaminate water supplies, disrupt ecosystems, and corrode vehicles and infrastructure (Pieper et al., 2018). Due to these issues, researchers and transportation departments have been exploring safer and more sustainable alternatives.
Management of icy roads
The management of icy roads is conducted through two distinct but complementary processes: anti-icing and de-icing. Anti-icing is a proactive approach where a liquid solution is applied to the pavement before snowfall occurs. Although effective under moderate snowfall conditions, anti-icing treatments are vulnerable to heavy precipitation and rapid temperature changes. High levels of snowfall can dilute or wash away the anti-icing products, rendering them less effective (Federal Highway Administration, 1996). Additionally, anti-icing effectiveness diminishes when temperatures drop below the eutectic point of the chemical solution being used, the lowest temperature at which the brine remains liquid. Below this threshold, the solution refreezes and loses its anti-icing capability. In such cases, de-icing becomes necessary. De-icing is a reactive process applied after snow or ice has bonded to the pavement. It involves the use of chemical agents or mechanical methods to break the ice-pavement bond, allowing for removal and restoring road safety in more severe winter conditions. While these methods are essential for maintaining road safety, their long-term effects introduce consequences that extend beyond immediate effectiveness, particularly in terms of environmental and infrastructural impacts.
Environmental concerns
While effective, anti-icing and de-icing chemicals such as magnesium chloride and sodium chloride pose several environmental and structural risks, as explained in Figure 1. For example, liquid magnesium chloride is ineffective below -15°C because it cannot lower the freezing point sufficiently. Moreover, when precipitation persists, road friction decreases drastically, increasing accident risks despite anti-icing measures (Mainroad, n.d.). Liquid brine—a 23% salt, 77% water solution—is more affordable and works in temperatures as low as -29°C, but corrodes infrastructure and pollutes ecosystems (Lilek, 2017; Mainroad, n.d.). NaCl harms freshwater species at just 100 mg/L and accumulates over time, degrading water quality (Corsi, De Cicco, Lutz, & Hirsch, 2015).
| Figure 1: Environmental and human impacts of road salt application. (Guidelines for the Selection, 2007) | 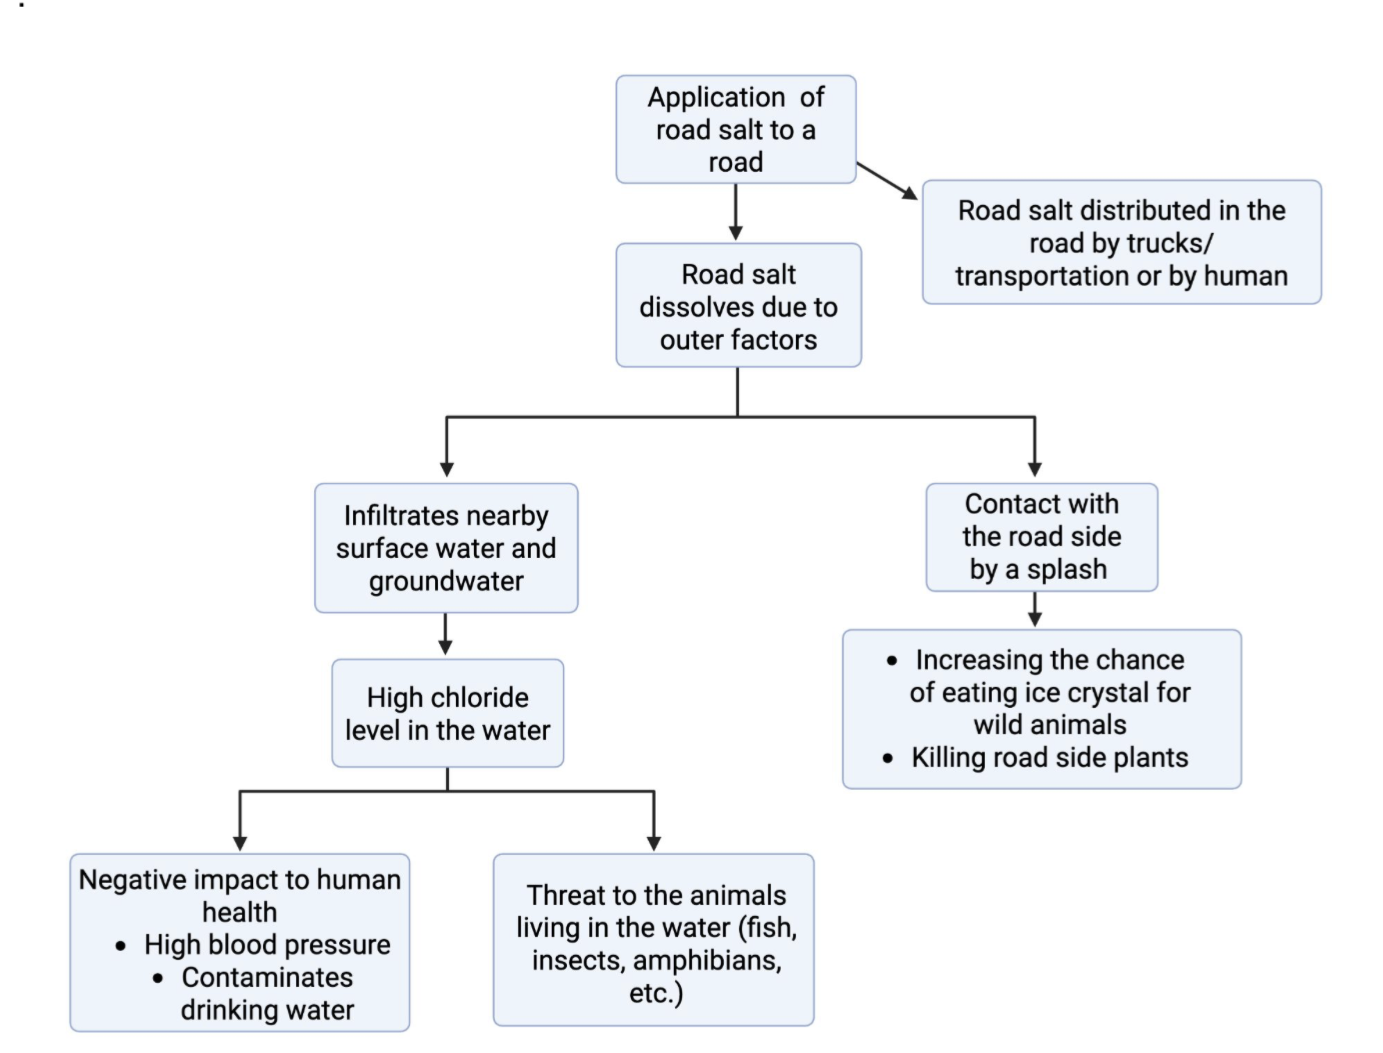 |
|---|
Cost
The most common product used in the de-icing step is road salt, primarily sodium chloride, due to its low cost, wide availability, and strong ability to lower the freezing point of water. Studies show the importance of de-icers in improving road surface conditions. In 2013, a mere 10% improvement in surface friction could lead to a 20% reduction in crashes. Road salt is the most affordable and efficient de-icer to ensure vehicle safety during winter (American Highway Users Alliance, 2018). American roads and highways use road salt, which has been proven to reduce collisions by up to 88% and injuries by 85%; on four-lane roads, this estimate is raised to 93% (American Highway Users Alliance, 2018).
The economic impact of road closures in the U.S. due to inclement weather, including costs associated with snow plowing and removal, is substantial. In Snow Belt states, the daily economic costs of statewide road closures due to winter weather can range from $300 to $700 million (American Highway Users Alliance, 2018). In this context, applying road salt represents a relatively modest investment. The cost of salt application pays for itself within the first four hours, as road users receive direct benefits of $6.50 for every $1.00 spent (American Highway Users Alliance, 2018). These benefits include reduced accident-related costs, improved traffic flow, and ultimately sustained economic activity during winter conditions.
Despite these strong short term economic benefits, the widespread use of road salt introduces significant long-term financial pressure that is often excluded from cost analysis, including infrastructure corrosion, increased vehicle maintenance costs, and rising expenses associated with freshwater treatment and environmental remediation.
As of today, road salt remains the most cost-effective option for ensuring road safety. However, these short-term economic benefits must be weighed against the long-term costs of infrastructure corrosion, environmental remediation, and water treatment, which are rarely considered in cost-benefit analysis. Also, the widespread use of chemical road salts has led to increasing concerns about soil and freshwater contamination and long-term environmental impact. Therefore, while road salt appears inexpensive at the point of application, its life-cycle cost may be substantially higher when indirect environmental and infrastructural costs are taken into account.
Our solution
The environmental contamination, health risks, and infrastructure costs of chloride-based de-icers establish a clear need for an alternative approach. Chloride ions are particularly problematic because they do not degrade. Once dissolved in runoff, chloride accumulates in soil and freshwater systems, with concentrations continuing to rise across all seasons and persisting long after the initial deposit (Corsi et al., 2015). This persistence drives the secondary costs that compound over successive years, including drinking water contamination, accelerated corrosion of vehicles and infrastructure, and chronic harm to freshwater species (Corsi et al., 2015; Pieper et al., 2018).
Antifreeze proteins (AFPs) offer a fundamentally different mechanism. AFPs are naturally occurring proteins that bind directly to ice surfaces and inhibit ice growth, achieving at micromolar concentrations what chemical salts require kilogram scale application to accomplish (Eskandari et al., 2020). Their advantages over chloride salts are threefold. First, AFPs do not corrode the metals and concrete used in vehicles and road infrastructure, eliminating the downstream maintenance costs associated with sodium chloride. Second, AFPs act at concentrations several orders of magnitude lower than road salts, so a small protein mass can treat a large surface area. Third, and most consequential for long term environmental impact, AFPs are biodegradable. As proteins, they break down into amino acids under standard environmental proteolytic activity, leaving no persistent ionic residue that bioaccumulates in soil or freshwater. In direct contrast to chloride, which remains chemically intact and continues to harm aquatic ecosystems long after the season of application, an AFP based de-icer is consumed and removed by the same biological processes that govern all organic matter in the environment.
This project applies the AFP approach by engineering E. coli to express two antifreeze proteins with complementary ice inhibition mechanisms. TmAFP from the mealworm beetle T. molitor and LpAFP from the perennial ryegrass L. perenne. T. molitor, a species of yellow mealworm beetle, generates two thermal hysteresis proteins (THPs), Cys-rich and Thr-rich (Graham et al., 2000). Thermal hysteresis refers to the phenomenon where the freezing point of a substance is lowered without interfering with its melting temperature (Eskandari et al., 2020). Thermal hysteresis proteins are types of antifreeze proteins (AFPs) that lower the freezing point of the hemolymph of T. molitor, enabling its survival in subzero temperatures. Organisms, including insects, fish, and plants, can synthesize THPs when they are exposed to environments where the temperature is consistently below 0°C (32°F). TmAFP is classified as a hyperactive insect AFP, featuring a β-helical structure with an extensive ice-binding surface that produces thermal hysteresis values of up to ~5°C, far exceeding the ~1°C typical of moderately active fish AFPs (Hakim et al., 2013). Importantly, T. molitor prevents ice from forming in body fluids by using AFPs employing a freeze-avoidance strategy rather than tolerating internal ice formation. This capacity to actively prevent ice formation, rather than survive its presence, makes TmAFP well-suited for road de-icing applications.
To complement TmAFP’s thermal hysteresis activity, a second AFP was selected from L. perenne. L. perenne produces an AFP (LpAFP) of approximately 118 amino acids featuring semi-conserved repeats folding into a β-roll structure that enables it to bind ice and inhibit ice crystal growth (Kuiper et al., 2001). Unlike TmAFP, which depresses the freezing point of ice through thermal hysteresis, LpAFP’s function is primarily ice recrystallization inhibition (IRI), preventing small ice crystals from merging into larger, more damaging formations (Pudney et al., 2003). Recent studies have shown that thermal hysteresis and IRI are driven by distinct ice-binding mechanisms (Tas et al., 2023), and that AFP mixtures with complementary ice-plane specificity can produce synergistic enhancement of activity (Berger et al., 2019). Insect AFPs such as TmAFP are typically an order of magnitude more active in freezing point depression, whereas plant AFPs such as LpAFP are more effective at IRI (Gruneberg et al., 2021). Together, TmAFP’s thermal hysteresis and LpAFP’s IRI activity target distinct stages of ice development. Although homologous domains have been identified in other Pooideae grasses such as wheat and barley, LpAFP is uniquely abundant in perennial ryegrass Expressed Sequence Tag and Bacterial Artificial Chromosome libraries, where some variants have demonstrated measurable ice-binding activity upon heterologous expression (Middleton et al., 2009). In plants, LpAFP has been stably integrated and transcribed in transgenic tomato lines (Balamurugan et al., 2018). Additionally, bacterial expression systems have yielded functional LpAFP that can be purified (Pudney et al., 2003). These studies highlight the practicality of expressing LpAFP genes in heterologous species.
AFPs prevent ice formation by first attaching to the ice surface, occupying the specific lattice positions where additional water molecules would otherwise attach and continue crystal growth (Eskandari et al., 2020). Ice crystals typically grow symmetrically and uniformly as water molecules continue to freeze. However, as detailed in Figure 2, the interference of binding AFPs alters this process by inducing the formation of a convex interface on the side facing the surrounding liquid (Hakim et al., 2013). This AFP-induced convexity changes the normal growth morphology of the ice crystal. According to the Gibbs-Thomson-Herring effect, those convex surfaces are thermodynamically less stable and unfavorable for further ice extension, as depicted in Figure 3, (Gharib et al., 2022).
| Figure 2: Mechanism of AFPs interfering with ice formation. Antifreeze proteins absorb onto the surface of an ice nucleus, forcing the crystal to grow with convex curvature between bound proteins, which is thermodynamically unfavorable and arrests further ice extension. Adapted from Kondo et al. (2012), as described in the SPring-8 press release (How a fungi-derived, 2012). Created in BioRender. Vacca, J. (2026) https://BioRender.com/ui9ezud | 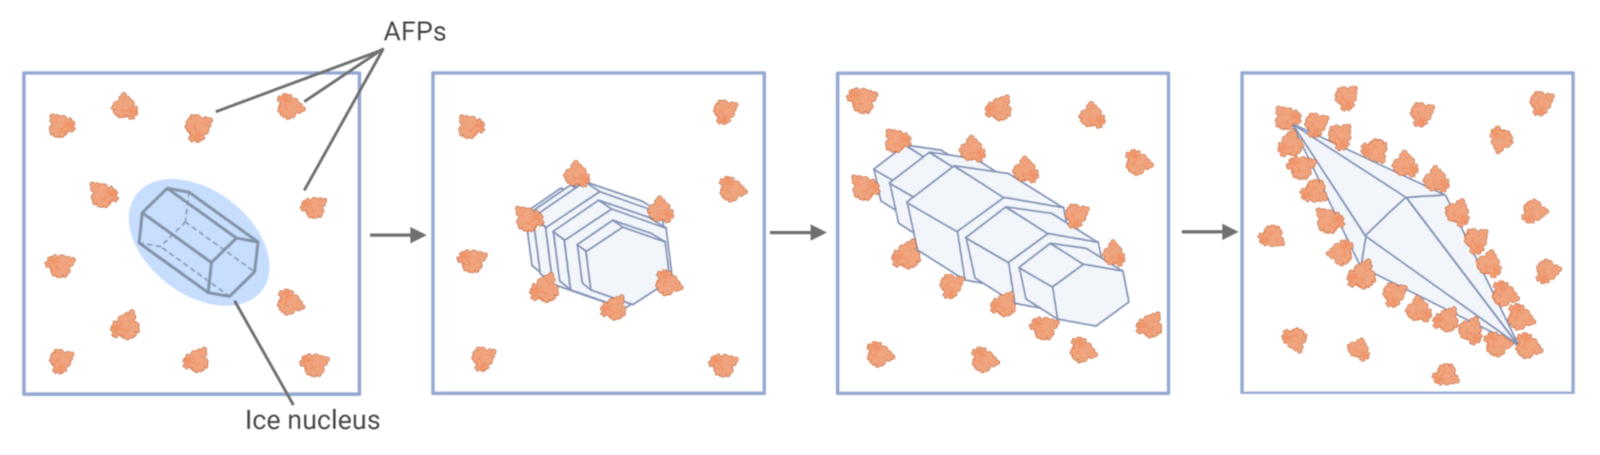 |
|---|
| Figure 3: Gibbs-Thomson-Herring effect and the mechanism of AFPs. (A) AFPs bind to the advancing ice front, while non-AFPs remain unbound. AFP binding increases the curvature of the ice surface, thereby inhibiting further ice growth (Kuiper et al., 2015). (B) A mixture of AFPs and non-AFPs near the ice front (Kuiper et al., 2015). Created in BioRender. Vacca, J. (2026) https://BioRender.com/h7gikli | 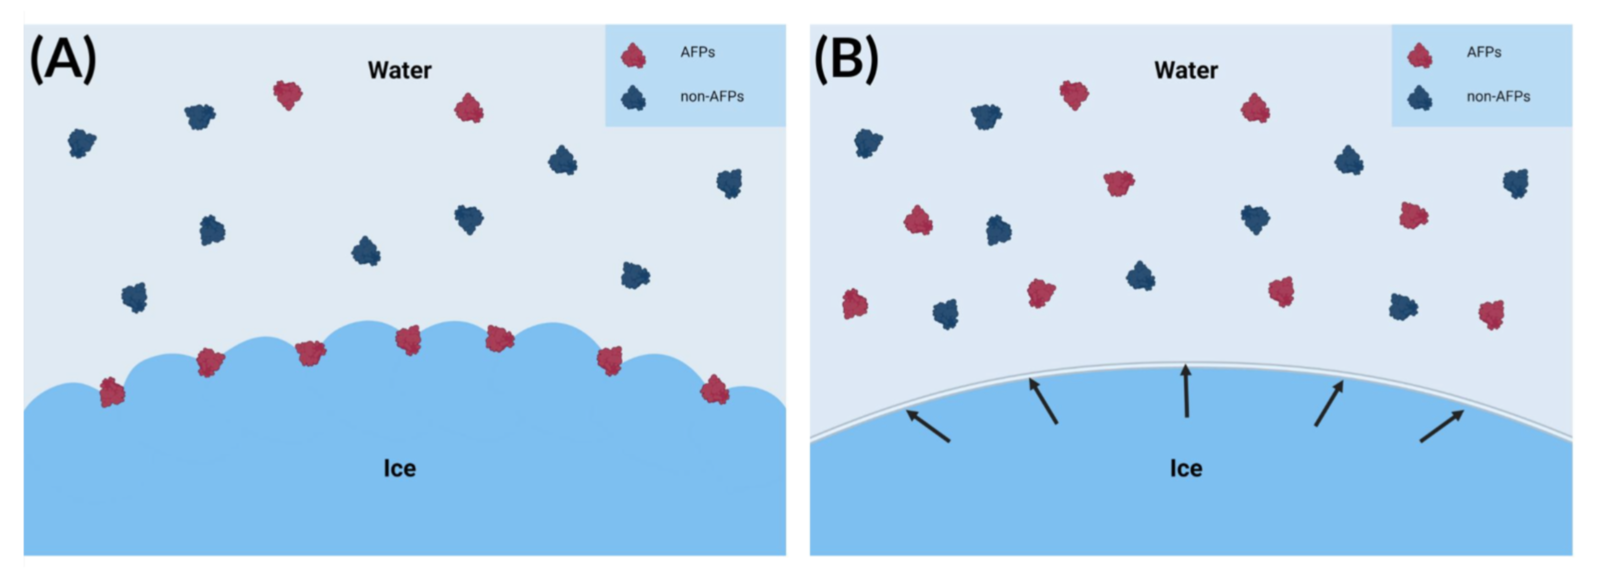 |
|---|
The structural types of AFP determine their ability to bind to specific crystallographic ice planes. This binding occurs through a region, known as the ice-binding site (IBS), on the AFP. The IBS is believed to organize water molecules adjacent to AFP into a conformation that mimics the lattice arrangement found in ice molecular structure, but without inducing actual ice formation (Kondo et al., 2012). By pre-arranging these water molecules into an ice-like pattern, AFPs effectively prepare their binding interface to complement a specific ice plane (Eskandari et al., 2020). The IBS then aligns with a corresponding plane on the ice surface upon encountering an ice crystal. The molecular complementarity between the water molecule arrangement at the IBS and the atomic structure of the targeted ice plane facilitates this attachment. Different AFPs exhibit different binding preferences depending on their structures. For instance, Type 1 AFPs from the winter flounder preferentially bind to the pyramidal and secondary prism planes of ice, whereas hyperactive AFPs from the Antarctic bacterium Flavobacterium frigoris PS1 target the basal plane of ice crystals (Kim et al., 2017). These matchings replace water binding that causes further ice crystal growth at the site and enables the AFP to selectively adhere to ice planes (Eskandari et al., 2020).
Thus, harnessing the precise ice‐plane specificity of AFPs offers a promising, biodegradable strategy for ice-prevention. Conventional de-icing agents pose environmental impacts, potential health hazards, and substantial economic costs, making the need to develop a more sustainable and cost-effective alternative pressing. By engineering an E. coli strain to produce AFPs derived from two specific sources, T. molitor and L. perenne, this project aims to utilize biodegradable AFPs to replace chemical road salts.
This team envisions our product as a mixture of two purified T. molitor AFP and LpAFP, formulated into an aqueous spray containing buffering agents, a food-grade surfactant to promote even spreading, and a stabilizer to preserve protein activity during storage and freezing. This reversible protein coating on pavement surfaces will bind nascent ice nuclei and prevent adherence without corroding underlying concrete or metal infrastructure.
Although AFP production is more expensive on a per-kilogram basis than bulk road salt, several factors could make our protein-based spray more cost-effective over its lifetime. With industrial fermentation of recombinant E. coli in optimized bioreactors using inexpensive carbon sources (e.g., glycerol or corn steep liquor), downstream costs for purified AFP can fall to the low tens of dollars per kilogram and continue to decline with process improvements and economies of scale (Puetz & Wurm, 2019). In addition, AFPs act at micromolar concentrations, so a single kilogram of protein can treat thousands of square meters of pavement versus one to two tons of salt per kilometer of road. By reducing corrosion and infrastructure repair costs, this bio-spray can generate net savings even at moderate protein production costs.
Previous data
In the initial phase of this project (Goyal et al., 2025), this team designed and constructed the two AFP expression plasmids, performed restriction enzyme cloning, and carried out preliminary transformations into E. coli DH5α. Both plasmid backbones, pBAD18-Kan and pUS212, were successfully isolated via miniprep and confirmed by spectrophotometry and agarose gel electrophoresis. Plasmid concentrations were 28.19 ng/μL (pBAD18-Kan, A260/A280 = 2.05) and 12.33 ng/μL (pUS212, A260/A280 = 1.57). Double Digestion with the cloning enzymes (NheI/SalI for LpAFP; SpeI/PstI for TmAFP) yielded fragments consistent with the expected sizes for both vectors and inserts, confirming successful restriction digestion.
Following ligation and heat shock transformation into DH5α, the TmAFP/pUS212 construct produced visible colonies on all chloramphenicol selective plates, with colony density increasing proportionally with plating volume. In contrast, the LpAFP/pBAD18-Kan construct yielded no colonies on any kanamycin selective plates despite parallel processing. This outcome suggested a construct specific issue, potentially in antibiotic selective conditions, rather than a general failure of the transformation protocol. These results established the TmAFP construct as ready for downstream screening and set the LpAFP construct as the primary troubleshooting target for the current phase of the project.
Materials and methods
Kanamycin stock solution preparation
6 LB agar plates were prepared (2 replicates per concentration) with kanamycin at final concentrations of 25, 35, and 50 µg/mL. A kanamycin stock solution was prepared by weighing 0.5 g of kanamycin powder (obtained from Goldbio) and dissolving it in 4 mL of distilled water (H2O), followed by the addition of 1 mL to adjust the concentration.
The kanamycin antibiotic solution was remade due to inaccuracies in measurement caused by an imprecise scale during the initial preparation. A new kanamycin stock solution was obtained, and the preparation process was repeated using the same volumes and procedures as previously described. During this step, additional research was conducted to confirm appropriate working concentrations for DH5α selection, ensuring that the final concentrations used (25–50 µg/mL) were within standard and effective ranges.
Kanamycin selective plates
For each plate, 12 mL of Luria Broth Agar (obtained from Evdotek) was used, and the corresponding volumes of kanamycin solutions were added to achieve the desired concentration: 0.1 mL for 25 µg/mL, 0.14 mL for 35 µg/mL, and 0.2 mL for 50 µg/mL.
Plating of DH5α transformed with pBAD18-Kan
DH5α cells transformed with pBAD18-Kan were plated onto kanamycin-selective LB plates using standard plating technique; 20 µL and 200 µL of the cell suspension were pipetted onto the surface of each pair of agar plates and evenly spread using a sterile spreader. The plates were then incubated at 37°C overnight to allow bacterial growth, and subsequently stored at 4°C to reduce the further spreading of colonies. However, as shown in Figure 4, the plates showed the formation of a bacterial lawn instead of distant, isolated colonies, suggesting overgrowth or ineffective antibiotic selection. This outcome was likely due to the reduced activity of kanamycin, potentially caused by improper preparation or heat inactivation during agar preparation.
| Figure 4: Confluent bacterial lawn on a kanamycin selective LB agar plate following plating of DH5α transformed with LpAFP/pBAD18-Kan. The plate contained kanamycin (25 µg/mL) prepared from GoldBio kanamycin powder. The absence of well-isolated colonies and the continuous bacterial lawn indicated that effective antibiotic selection was not achieved, suggesting that the prepared kanamycin stock was insufficiently concentrated or had been inactivated during plate preparation. | 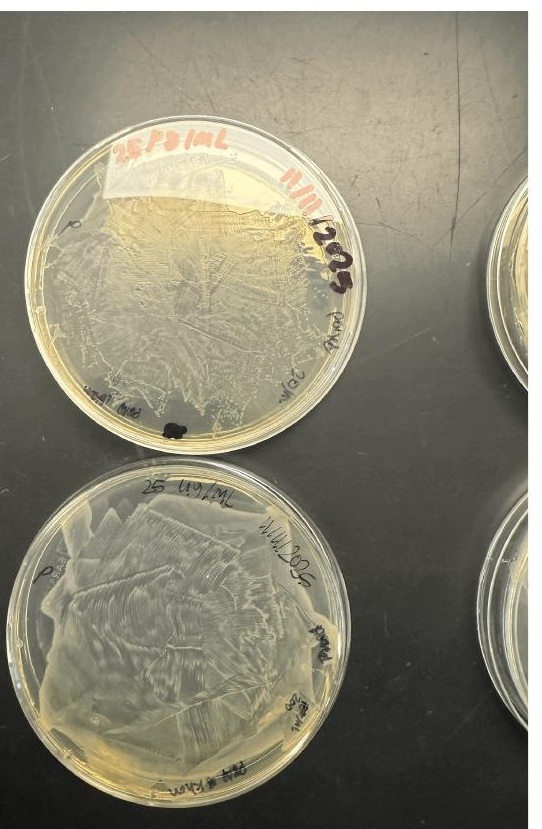 |
|---|
New selective plates were poured at the same concentrations due to the lack of well-isolated colonies. The plating procedure was repeated under the same conditions as the initial attempt. Despite using a freshly prepared antibiotic stock, confluent bacterial lawns were again observed, with no isolated colonies obtained for the LpAFP/pBAD18-Kan construct. Based on these repeated results, a commercially prepared kanamycin solution (Carolina Biological) was ordered for all subsequent experiments.
Kanamycin Antibiotic Selective Plates with Commercially Available Kanamycin Solution
Due to inconsistencies using kanamycin powder (GoldBio) to produce kanamycin solution, a new set of kanamycin selective LB agar plates was prepared using a commercially obtained kanamycin solution (Carolina Biological 10 mg/mL). For each plate, 12 mL of ReadyPour LB/Agar Base (Carolina Biological) was melted and cooled to 50-55°C, and kanamycin was added to a final working concentration of 50 µg/mL by pipetting 60 µL of the 10 mg/mL stock solution into the molten agar. The plates were allowed to solidify at room temperature then transferred to 4°C.
Chloramphenicol antibiotic solution
A chloramphenicol antibiotic stock solution was prepared by dissolving chloramphenicol powder in 70% ethanol, due to its low solubility in water. The solution was mixed thoroughly until fully dissolved. The stock was then stored at -20°C, and later diluted to the appropriate working concentration for selective plating.
Chloramphenicol antibiotic selective plates
A chloramphenicol stock solution (10 mg/mL in 70% ethanol) was used to prepare selective media. To achieve a final concentration of 34 µg/mL, 3.4 µL of the stock solution was added per 1 mL of broth. For the total volume prepared, 41 µL of chloramphenicol stock was added per plate and mixed thoroughly to ensure even distribution before use.
Bacterial recovery phase
To recover bacterial cells from frozen stocks, an aliquot was taken and inoculated into LB medium containing the appropriate antibiotic. The culture was incubated at 37°C with shaking in a loosely capped tube to allow aeration, and grown overnight (~16 h). The recovered culture was then used for subsequent plating onto selective agar plates.
Plating of DH5α transformed with pUS212 and DH5α transformed with pBAD18-Kan
Following overnight recovery DH5α cells transformed with the TmAFP genes in pUS212 were plated onto chloramphenicol selective plates, and DH5α cells transformed with the LpAFP genes in pBAD18-Kan were plated onto kanamycin selective plates. Plates were incubated at 37°C overnight and then transferred to 4°C.
Bacterial cells incubated in LB with kanamycin and chloramphenicol
Cells from the TmAFP pUS212 chloramphenicol selective plates were inoculated into LB broth (Carolina Biological) supplemented with chloramphenicol at a working concentration of 34 µg/mL. Cultures were incubated at 37°C with shaking overnight to maintain antibiotic selection pressure throughout the liquid outgrowth, ensuring that only plasmid-bearing cells survived. LpAFP pBAD18-Kan liquid cultures were similarly inoculated in LB broth supplemented with kanamycin at 50 µg/mL. Although no isolated colonies were obtained for either construct, visible growth and clouding of culture media were observed across all stages at which antibiotic selection pressure was maintained, including recovery in SOC medium with antibiotic, liquid outgrowth in selective LB, and plating on selective agar. This persistent growth under continuous selection suggests that the surviving cells likely harbor their respective resistance plasmids, though formal verification by colony polymerase chain reaction (PCR) is required.
Cryopreservation
For cryopreservation, a sample of the confluent lawn was harvested using a sterile pipette tip and inoculated into 5 mL of LB broth containing the appropriate antibiotic for the corresponding plasmid. The culture was incubated overnight at 37°C with shaking (~200 RPM) until it reached visible turbidity, indicating sufficient bacterial growth. To prepare the glycerol stock, 500 µL of the overnight culture was combined with 500 µL of sterile 50% glycerol to achieve a final glycerol concentration of 25%. The mixture was gently homogenized by pipetting, then stored at -80°C for long-term preservation.
Results
Kanamycin plate optimization and initial LpAFP plating
To address the lack of LpAFP colonies observed in the prior year, kanamycin selective plates were prepared at three concentrations (25, 35, and 50 µg/mL) with two replicate plates per concentration. DH5α cells transformed with LpAFP/pBAD18-Kan were plated on all six plates and incubated at 37°C overnight. All plates, including those at the lowest kanamycin concentration (25 µg/mL), displayed confluent bacterial lawns rather than isolated colonies. The absence of defined colonies across all concentrations suggested that the antibiotic was not providing effective selection, raising the possibility that the prepared kanamycin stock was insufficiently concentrated or had been inactivated during preparation.
Repeated plating with remade kanamycin stock
A second kanamycin stock solution was prepared, and the plating procedure was repeated under identical conditions. Confluent bacterial lawns were again observed across all plates, as shown in Figure 5, reproducing the results of the initial attempt. Because the same outcome occurred with independently prepared antibiotic stocks, we transitioned to a commercially prepared kanamycin solution (Carolina Biological, 10 mg/mL) for subsequent experiments.
| Figure 5: Six kanamycin selective LB agar plates from the second plating attempt using an independently prepared kanamycin stock. Plates contained kanamycin at 25, 35, and 50 µg/mL (two replicates per concentration) and were inoculated with DH5α transformed with LpAFP/pBAD18-Kan. The two plates on the left contain 25 µg/mL kanamycin, the two middle plates contain 35 µg/mL, and the two plates on the right contain 50 µg/mL. Confluent bacterial lawns were observed across all six plates regardless of antibiotic concentration, reproducing the outcome of the initial attempt and prompting the transition to a commercially prepared kanamycin solution for subsequent work. | 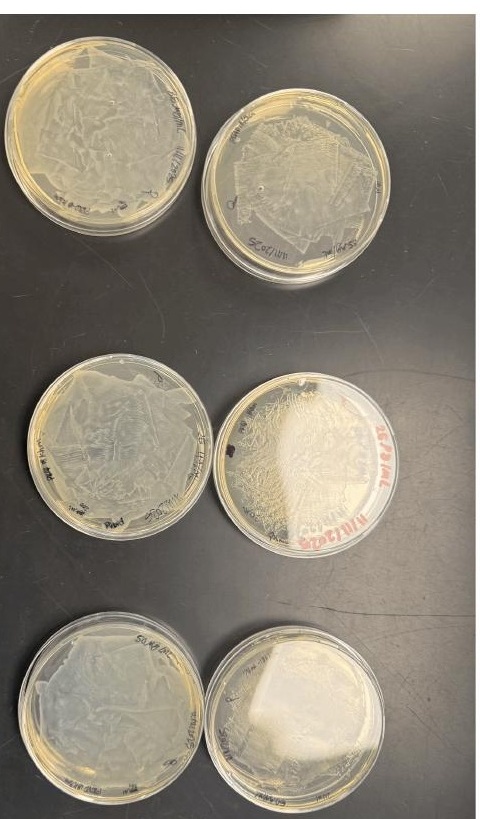 |
|---|
Recovery and plating with chloramphenicol and commercial kanamycin
Following the transition to the commercial kanamycin solution, a recovery step was performed. Transformed DH5α cells carrying either LpAFP/pBAD18-Kan or TmAFP/pUS212 were recovered overnight in SOC medium supplemented with the appropriate antibiotic. After recovery, cells were plated on selective agar plates prepared with the commercial kanamycin (50 µg/mL) or chloramphenicol (34 µg/mL). Plating was performed using a standard spread plate technique with a sterile spreader. Neither construct yielded isolated, well-defined colonies; both plates again showed confluent growth, as shown in Figure 6.
| Figure 6: Selective LB agar plates following overnight liquid recovery in SOC medium under antibiotic selection. The left plate is a chloramphenicol selective plate (34 µg/mL) inoculated with DH5α transformed with TmAFP/pUS212; the right plate is a kanamycin selective plate (50 µg/mL, Carolina Biological commercial solution) inoculated with DH5α transformed with LpAFP/pBAD18-Kan. Both plates exhibited confluent growth rather than isolated colonies, although the sustained growth under continuous antibiotic selection across all stages of the workflow suggested that the surviving cells likely retained their respective resistance plasmids. | 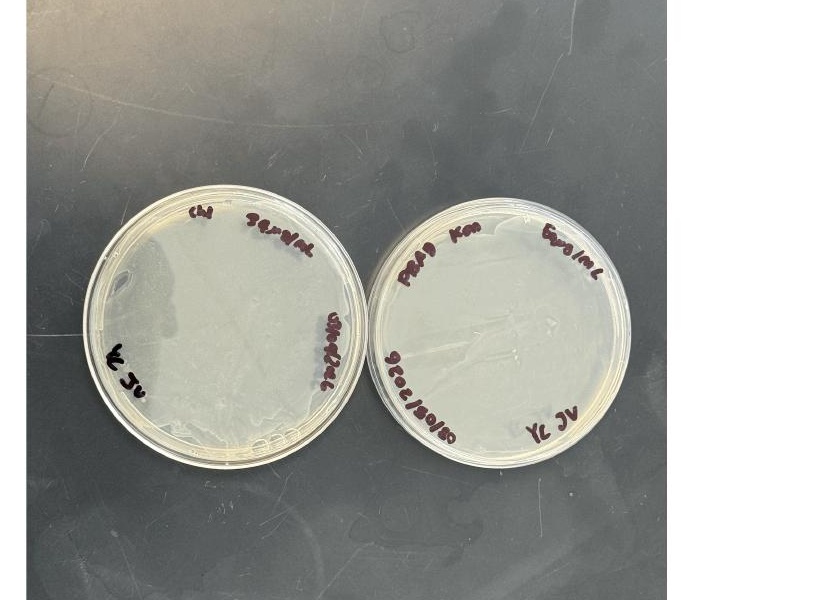 |
|---|
Evidence of plasmid retention under selection
Although no isolated colonies were obtained for either construct, visible growth and turbidity were consistently observed at every stage at which antibiotic selection pressure was maintained, during overnight recovery in SOC medium with antibiotics, liquid outgrowth in selective LB broth, and on selective agar plates. Because non-transformed DH5α cells lack intrinsic resistance to kanamycin or chloramphenicol, this persistent growth under continuous antibiotic selection suggests that the surviving cells likely harbor their respective resistance plasmids. However, formal verification by colony PCR is required to confirm the presence and correct orientation of the AFP inserts. The inability to obtain isolated colonies may reflect high transformation efficiency leading to dense plating, residual satellite colony growth, or incomplete antibiotic distribution during plate preparation.
Cryopreservation
Cells from overnight liquid cultures grown under antibiotic selection were cryopreserved in 25% glycerol solution at -80°C. These stocks were labeled as “unconfirmed” pending the colony PCR verification described above.
Discussions
This report describes the second phase of an ongoing effort to engineer E. coli to express antifreeze proteins from T. molitor and L. perenne as an environmentally friendly alternative to chemical road salt. Earlier work in this project established both expression plasmids, verified the backbones by spectrophotometry and restriction digest, and carried out heat shock transformations into E. coli DH5α, producing reproducible growth for TmAFP/pUS212 on chloramphenicol selective media but no growth for LpAFP/pBAD18-Kan on kanamycin selective media (Goyal et al., 2025). The LpAFP transformation failure was identified as the principal unresolved bottleneck at the start of the present phase. The results reported here advance that work by establishing conditions under which both constructs produce sustained growth under continuous antibiotic selection, while simultaneously identifying the molecular characterization steps that remain outstanding before either construct can be used for recombinant protein expression.
The main observation of this phase is that DH5α cultures carrying either construct now produce dense, confluent growth on selective media rather than discrete, well-isolated colonies typically obtained from successful transformation. Because untransformed DH5α lacks intrinsic resistance to either kanamycin or chloramphenicol, growth sustained across the full workflow, including recovery in selective SOC, overnight outgrowth in selective LB, and plating on selective agar, is most easily explained by the presence of resistance-conferring plasmids in the surviving population. This interpretation is further supported by the observation of visible turbidity at every stage at which selection pressure was maintained, including in media freshly inoculated from cryopreserved stocks. Several nonexclusive factors likely contribute to the confluent rather than discrete colony morphology, including high transformant density, plating volumes used, and satellite colony formation permitted by localized antibiotic degradation within the agar. None of these alternatives contradict the inference that the cultures contain plasmid-bearing cells, but all of them preclude the isolation of single clonal lineages, which is a prerequisite for downstream verification and expression work. A further limitation of the current results is the absence of two controls that would strengthen this interpretation: untransformed DH5α plated on the same selective media, which would confirm that the antibiotic is excluding non-resistant cells, and DH5α transformed with an empty backbone, which would establish baseline transformation efficiency under the current protocol. Without these controls, the alternative explanation that the confluent growth reflects insufficient antibiotic activity rather than successful transformations cannot be formally excluded.
The LpAFP/pBAD18-Kan result is of particular significance to the project’s trajectory. Two successive kanamycin stocks failed to support growth consistent with effective antibiotic selection, a pattern that mirrored the null outcome for this construct reported previously (Goyal et al., 2025). Substitution of a commercially standardized kanamycin solution, combined with the addition of an overnight liquid recovery step under selection, produced the first sustained growth reported for the LpAFP construct in this project. This outcome suggests that the earlier failure was most likely attributable to insufficient antibiotic activity in the prepared selection medium rather than to a defect in the ligated plasmid itself, and it shifts the LpAFP construct from a complete failure of selection to a verifiable starting point for colony isolation and molecular characterization.
Several important verifications remain before the results reported here can be interpreted as successful construct assembly. Growth under antibiotic selection is a necessary but not sufficient criterion for correct cloning, and colony PCR, along with diagnostic restriction digestion where feasible, is required to confirm that the AFP inserts are present in the expected orientation and free of mutations introduced during ligation or transformation. In addition, all work to date has been conducted in DH5α, an optimized cloning strain whose genotype is not suited to the arabinose-inducible recombinant protein expression ultimately required for this project. Transformation into the BL21 expression strain is therefore a prerequisite for any downstream functional assay. Finally, the glycerol stocks generated in this phase were labeled as unconfirmed and should be regarded as provisional, to be replaced with a second, PCR-verified set before being used as source material for expression work.
Despite these limitations, the results reported here represent a meaningful advance relative to the prior phase of the project. The complementary anti-icing activities described in the Background, consisting of thermal hysteresis from TmAFP paired with IRI from LpAFP (Berger et al., 2019; Gruneberg et al., 2021; Tas et al., 2023), cannot be evaluated until both proteins can be reliably produced and purified.
Next steps
Following the successful preparation of selective plates and initial bacterial growth, our team will first serially dilute the confluent bacterial cultures and apply a four-quadrant streaking technique on fresh selective agar to obtain discrete, well-isolated colonies. The four-quadrant approach progressively reduces cell density across each successive quadrant, increasing the likelihood that the final quadrant yields physically separated colonies suitable for downstream picking and colony PCR screening. In parallel, all subsequent transformations will include two control plates per antibiotic condition. The first is an untransformed DH5α plated on the selective medium, which should show no growth if that antibiotic concentration is sufficient to exclude non-resistant cells. The second is DH5α transformed with the empty vector backbone (pBAD18-Kan or pUS212 with no AFP insert), which should show growth if transformation and selection are functioning as expected. Together, these controls will distinguish failures of transformation from failures of antibiotic selection in any future construct work. After isolated colonies are obtained, several well-isolated colonies from the pBAD18-Kan and pUS212 plates will be inoculated into 3-5 mL of liquid LB broth supplemented with their appropriate antibiotic, kanamycin for pBAD18-Kan and chloramphenicol for pUS212.
After overnight growth at 37°C in a shaking incubator, the plasmid DNA will be isolated using miniprep to obtain a purified template for downstream verification. To confirm that these colonies contain the correct construct rather than an empty vector, failed ligation product, or an incorrect plasmid arrangement, our team will perform PCR using primers designed either within the insert or flanking the cloning site. The amplified products will then be analyzed by agarose gel electrophoresis, where the observed band sizes will be compared to the expected fragment lengths for each construct. Colonies that produce the correct PCR band will be considered positive candidates for successful amplification.
Once positive colonies are identified, our team will expand the confirmed cultures and perform an additional miniprep to obtain a larger quantity of plasmid DNA for further validation. These plasmids may then be used for sequencing to verify that the insert is present in the correct orientation and that no unintended mutations were introduced during cloning. After sequence confirmation, the validated constructs will be transformed into an expression strain for protein production. Recombinant expression of disulfide-rich insect AFPs such as TmAFP in E. coli is known to be complicated by misfolding in the reducing cytoplasm of standard expression strains (Hakim et al., 2013). To address this, predicted structures of the expressed proteins will be generated using AlphaFold and compared to published reference structures for TmAFP (Hakim et al., 2013) and LpAFP (Kuiper et al., 2001; Middleton et al., 2009) before functional testing. If misfolding is indicated by either the structural comparison or initial activity assays, the team will consider switching to an oxidizing-cytoplasm expression strain such as SHuffle T7, co-expressing disulfide isomerase chaperones, or refolding the proteins from inclusion bodies using established products. In the longer term, the expressed antifreeze proteins will be purified to evaluate whether each construct produces sufficient and stable protein for downstream analysis. Purified protein samples will then be used in future experiments to assess expression quality, compare construct performance, and support eventual functional testing of antifreeze activity.
Functional validation of AFP activity will use established cryobiological assays, including the splat-cooling assay for IRI and nanoliter osmometry or differential scanning calorimetry for thermal hysteresis measurement. For eventual deployment, considerations including plasmid stability across generations under industrial fermentation, the use of auxotrophic or kill-switch biocontainment strains, and protein purification from the bacterial chassis rather than direct release of engineered organisms will be required.
Author contributions
JV worked on the initial lab report, inspiring this project. JV and YC collaborated to write and revise the Background, Materials and methods, Results, Discussion, and Next steps. JV worked to create Figures 1-3.
Acknowledgements
We gratefully acknowledge the Western Reserve Academy Science Department for providing funding and oversight for this project. We are especially thankful to Ms. Marmerstein for her guidance and support throughout the research process. We also extend our sincere gratitude to our mentor, Dr. Meyer, for her insightful advice and encouragement. Finally, we extend our appreciation to BioBuilder for fostering our work in synthetic biology and to BioTreks for the opportunity to share our research through peer review and publication
References
American Highway Users Alliance. (2018). Road salt: A primer on the factors affecting supply and demand. https://www.highways.org/wp-content/uploads/2018/12/road-salt-primer-2018.pdf
Balamurugan, S., Ann, J. S., Varghese, I. P., Murugan, S. B., Harish, M. C., Kumar, S. R., & Sathishkumar, R. (2018). Heterologous expression of Lolium perenne antifreeze protein confers chilling tolerance in tomato. Journal of Integrative Agriculture, 17(5), 1128–1136. https://doi.org/10.1016/s2095-3119(17)61735-0
Berger, T., Meister, K., DeVries, A. L., Eves, R., Davies, P. L., & Drori, R. (2019). Synergy between antifreeze proteins is driven by complementary ice-binding. Journal of the American Chemical Society, 141(48), 19144–19150. https://doi.org/10.1021/jacs.9b10905
Cary Institute of Ecosystem Studies. (n.d.). It makes our roads safer, but is polluting our waterways. https://www.caryinstitute.org/our-expertise/freshwater/road-salt
Corsi, S. R., De Cicco, L. A., Lutz, M. A., & Hirsch, R. M. (2015). River chloride trends in snow-affected urban watersheds: Increasing concentrations outpace urban growth rate and are common among all seasons. Science of the Total Environment, 508, 488–497. https://doi.org/10.1016/j.scitotenv.2014.12.012
Eskandari, A., Leow, T. C., Rahman, M. B. A., & Oslan, S. N. (2020). Antifreeze proteins and their practical utilization in industry, medicine, and agriculture. Biomolecules, 10(12), 1649. https://doi.org/10.3390/biom10121649
Federal Highway Administration. (1996). Manual of practice for an effective anti-icing program: A guide for highway winter maintenance personnel. U.S. Department of Transportation. https://www.fhwa.dot.gov/publications/research/safety/95202/002.cfm
Gharib, G., Saeidiharzand, S., Sadaghiani, A. K., & Koşar, A. (2022). Antifreeze proteins: A tale of evolution from origin to energy applications. Frontiers in Bioengineering and Biotechnology, 9, 770588. https://doi.org/10.3389/fbioe.2021.770588
Goyal, A., Pae, N., Vacca, J., & Wang, L. (2025). Engineering Escherichia coli to produce Tenebrio molitor and Lolium perenne antifreeze proteins as a road salt alternative. BioTreks, 8, 43–56, e202504. https://biotreks.org/e202504/
Graham, L. A., Walker, V. K., & Davies, P. L. (2000). Developmental and environmental regulation of antifreeze proteins in the mealworm beetle Tenebrio molitor. European Journal of Biochemistry, 267(21), 6452–6458. https://doi.org/10.1046/j.1432-1327.2000.01734.x
Gruneberg, A. K., Graham, L. A., Eves, R., Agrawal, P., Oleschuk, R. D., & Davies, P. L. (2021). Ice recrystallization inhibition activity varies with ice-binding protein type and does not correlate with thermal hysteresis. Cryobiology, 99, 28–39. https://doi.org/10.1016/j.cryobiol.2021.01.017
Guidelines for the selection of snow and ice control materials to mitigate environmental impacts. (2007). Transportation Research Board. https://doi.org/10.17226/23178
Hakim, A., Nguyen, J. B., Basu, K., Zhu, D. F., Thakral, D., Davies, P. L., Isaacs, F. J., Modis, Y., & Meng, W. (2013). Crystal structure of an insect antifreeze protein and its implications for ice binding. Journal of Biological Chemistry, 288(17), 12295–12304. https://doi.org/10.1074/jbc.m113.450973
How a fungi-derived antifreeze protein works: Elucidation of molecular structure and antifreeze mechanism [Press release]. (2012, May 29). SPring-8. http://www.spring8.or.jp/en/news_publications/press_release/2012/120529/
Kim, H., Lee, J., Hur, Y., Lee, C., Park, S.-H., & Koo, B.-W. (2017). Marine antifreeze proteins: Structure, function, and application to cryopreservation as a potential cryoprotectant. Marine Drugs, 15(2), 27. https://doi.org/10.3390/md15020027
Kondo, H., Hanada, Y., Sugimoto, H., Hoshino, T., Garnham, C. P., Davies, P. L., & Tsuda, S. (2012). Ice-binding site of snow mold fungus antifreeze protein deviates from structural regularity and high conservation. Proceedings of the National Academy of Sciences, 109(24), 9360–9365. https://doi.org/10.1073/pnas.1121607109
Kuiper, M. J., Davies, P. L., & Walker, V. K. (2001). A theoretical model of a plant antifreeze protein from Lolium perenne. Biophysical Journal, 81(6), 3560–3565. https://doi.org/10.1016/s0006-3495(01)75986-3
Kuiper, M. J., Morton, C. J., Abraham, S. E., & Gray-Weale, A. (2015). The biological function of an insect antifreeze protein simulated by molecular dynamics. eLife, 4, e05142. https://doi.org/10.7554/eLife.05142
Lilek, J. (2017, July 13). Roadway deicing in the United States [Fact sheet]. American Geosciences Institute. https://www.americangeosciences.org/geoscience-currents/roadway-deicing-united-states
Mainroad liquid anti-icing brine program. (n.d.). Mainroad. https://mainroad.ca/mainroad-liquid-anti-icing-brine-program-faq/
Middleton, A. J., Brown, A. M., Davies, P. L., & Walker, V. K. (2009). Identification of the ice-binding face of a plant antifreeze protein. FEBS Letters, 583(4), 815–819. https://doi.org/10.1016/j.febslet.2009.01.035
Pieper, K. J., Tang, M., Jones, C. N., Weiss, S., Greene, A., Mohsin, H., Parks, J., & Edwards, M. A. (2018). Impact of road salt on drinking water quality and infrastructure corrosion in private wells. Environmental Science & Technology, 52(24), 14078–14087. https://doi.org/10.1021/acs.est.8b04709
Pudney, P., Buckley, S., Sidebottom, C., Twigg, S., Sevilla, M.-P., Holt, C., Roper, D., Telford, J., McArthur, A., & Lillford, P. (2003). The physico-chemical characterization of a boiling stable antifreeze protein from a perennial grass (Lolium perenne). Archives of Biochemistry and Biophysics, 410(2), 238–245. https://doi.org/10.1016/s0003-9861(02)00697-5
Puetz, J., & Wurm, F. M. (2019). Recombinant proteins for industrial versus pharmaceutical purposes: A review of process and pricing. Processes, 7(8), 476. https://doi.org/10.3390/pr7080476
Tas, R. P., Hendrix, M. M. R., & Voets, I. K. (2023). Nanoscopy of single antifreeze proteins reveals that reversible ice binding is sufficient for ice recrystallization inhibition but not thermal hysteresis. Proceedings of the National Academy of Sciences, 120(2), e2212456120. https://doi.org/10.1073/pnas.2212456120